


The Molecular Clock: From Random Mutations to Measuring Time
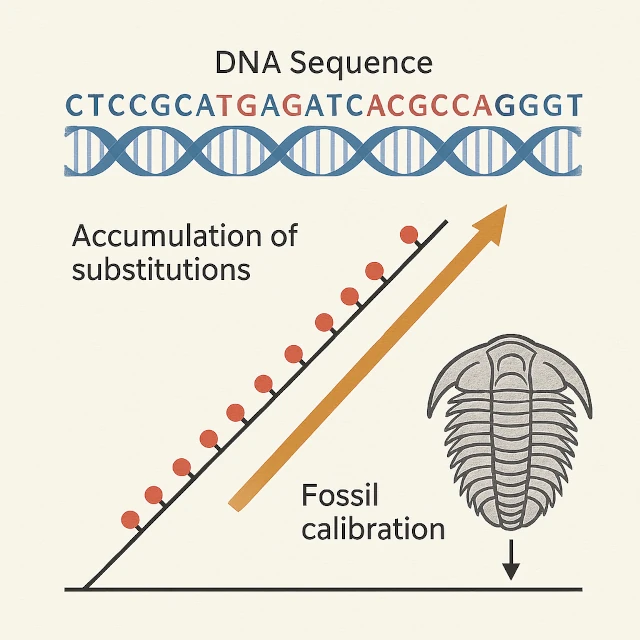
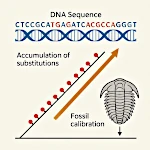
conceptual diagram showing a DNA sequence, the accumulation of substitutions, and calibration by fossil.
Image source: astronoo.com (new window)
What is the molecular clock and how does it allow dating of evolutionary events?
The molecular clock is a concept in evolutionary biology that estimates the time since the divergence of two lineages (species, populations) by measuring the genetic differences accumulated in their genomes. The principle relies on the accumulation of neutral substitutions (mutations with no effect on survival or reproduction) at a relatively constant rate over time. The relationship is: T = D / (2μ), where T is divergence time, D is genetic distance (proportion of differences between homologous sequences), and μ is the mutation rate. This method has dated major events: human-chimpanzee divergence (~6-8 Ma), Homo sapiens out-of-Africa (~60,000-100,000 years), dog domestication (~15,000-40,000 years), and the emergence of SARS-CoV-2 (2019).
Principle of the Molecular Clock
The molecular clock (molecular Clock) is a revolutionary concept in evolutionary biology that allows dating speciation events by using the rate of mutation accumulation in the genome.
The term "molecular clock" refers to the ability to estimate the time elapsed since the divergence of two lineages by measuring the amount of differences accumulated in their biomolecular sequences. The principle is based on the idea that neutral substitutions accumulate at an average rate, which can be used as a chronometer.
N.B.:
A neutral substitution is a change in the DNA or protein sequence that has no effect on the survival or reproduction of the organism.
These substitutions are neither favored nor eliminated by natural selection and therefore accumulate randomly over time.
In its simplest form, the relationship between divergence and time is given by \(T = \dfrac{D}{2\mu}\).
Parameters of the Molecular Clock
| Symbol | Name | Unit | Physical meaning |
|---|---|---|---|
| \(T\) | Divergence time | years (or Ma) | Time elapsed since two lineages diverged from a common ancestor; this is the measure of time that the molecular clock allows to estimate. |
| \(D\) | Genetic distance | substitutions/site | Average proportion of differences accumulated between two homologous sequences since their separation; reflects the number of substitutions neutralized by independent evolution in each lineage. |
| \(\mu\) | Mutation rate | substitutions/site/year | Frequency at which a particular base is replaced by another over a unit of time in a lineage; this is the speed of the molecular clock. |
N.B.:
In evolutionary biology, a lineage refers to a set of organisms descending from one another through reproduction, forming a continuous chain over time.
In the context of the molecular clock (model for estimating the time elapsed since an evolutionary divergence), each lineage independently accumulates substitutions, and the genetic distance \(D\) between two lineages corresponds to the sum of changes that have occurred in each since their last common ancestor.
Applications and Key Datings
The molecular clock has revolutionized our understanding of evolution by allowing precise dating of key events in the history of life, from divergences between major taxonomic groups to recent evolutionary events.
It has notably resolved long-standing debates on the chronology of evolution and provided temporal frameworks for phenomena as varied as the emergence of new species, human migrations, the origin of pandemics, and the domestication of species.
Key datings of evolution by genetic analysis
| Divergence event | Estimated time | Genetic material used | Reliability |
|---|---|---|---|
| Eukaryotes - Prokaryotes | 2-3 billion years | Ribosomal genes | Moderate |
| Origin of photosynthesis | 2.5-3.2 billion years | Photosynthetic genes | Moderate |
| Mammals - Birds | 310 million years | Conserved genes | Medium |
| Origin of flowering plants | 300 million years | Chloroplast genes | Medium |
| Radiation (rapid diversification) of dinosaurs | 230-250 million years | Skeletal genes | Moderate |
| Divergence birds - crocodilians | 240-275 million years | Nuclear genes | Medium |
| Radiation (rapid diversification) of placental mammals | 66-100 million years | Mitochondrial and nuclear DNA | Medium |
| Cetaceans - Hippopotamuses | 50-60 million years | Nuclear genes | High |
| Human - Chimpanzee | 6-8 million years | Nuclear and mitochondrial genome | High |
| Mouse - Rat | 12-24 million years | Complete genome | High |
| Neanderthal - Modern Human divergence | 550,000-765,000 years | Ancient nuclear genome | High |
| Domestication of the dog | 15,000-40,000 years | Mitochondrial DNA | Medium |
| Colonization of the Americas | 15,000-20,000 years | Complete human genome | High |
| Out of Africa migration of Homo sapiens | 60,000-100,000 years | Mitochondrial DNA and Y chromosome | High |
| Domestication of rice | 8,000-13,000 years | Chloroplast genome | High |
| Emergence of HIV-1 | Early 20th century | Complete viral genome | High |
| Emergence of SARS-CoV-2 | 2019 | Complete viral genome | High |
- Additional sources and tools: PubMed / NCBI (new window), BEAST (Bayesian clocks) (new window), Scientific literature (new window).
Limitations and Challenges
Despite its power, the molecular clock has several important limitations:
- Calibration: Depends on the quality of fossil data
- Variable rates: The mutation rate is not constant between lineages
- Saturation: Over long periods, the same sites can mutate multiple times
- Natural selection: Can bias the accumulation of neutral mutations
- Source: Nature - The molecular clock and evolutionary relationships (new window) and Science - Molecular Clocks in Evolution (new window).
FAQ: Everything about the molecular clock
What is a "neutral substitution" and why is it central to the molecular clock's function?
A neutral substitution is a point mutation in a DNA or protein sequence that has no effect on the organism's survival or reproduction. These mutations are neither favored nor eliminated by natural selection; they accumulate randomly and regularly over time, like "pencil marks" on a text. It is this statistical regularity that allows neutral substitutions to be used as a molecular "stopwatch": the longer two lineages have diverged, the more neutral differences they have accumulated in their genomes.
How do scientists "calibrate" the molecular clock?
Calibration of the molecular clock relies on independent temporal reference points, primarily provided by fossils. For example, if the oldest known fossil of a group (e.g., placental mammals) dates to about 66 million years, this age is used as a calibration point to calculate the mutation rate μ (substitutions per site per year). The genetic distance D measured between two species is divided by 2×T (where T is the known divergence time) to obtain μ. This calibrated rate is then applied to other groups to estimate their divergence times. Modern methods use Bayesian models that integrate multiple fossils and account for rate variations between lineages.
What are the main limitations of the molecular clock?
The molecular clock has several important limitations: 1) calibration dependence: the quality of dating relies on the reliability of fossils used as reference points; 2) variable mutation rates: the mutation rate is not constant across lineages (it can vary by species, generation time, or selection pressures); 3) saturation: over very long time periods, the same sites can mutate multiple times, erasing accumulated differences; 4) natural selection: can bias mutation accumulation if some mutations are beneficial or harmful. Modern methods (Bayesian clocks, variable-rate models) attempt to correct these biases.
 From the Zeroth Law to Generative AI: Asimov's Laws in Question
 How do complex societies emerge and disappear?
 The Brain vs. AI: Chronicle of an Organ Overwhelmed by the Data Deluge
 AI has learned to think: will artificial consciousness learn to be?
 The Future Obsession: When prediction shapes the living
 Which Regions of the World Will Remain Habitable During the Next Ice Age?
 Rapid Evolution: Darwin’s Thunderbolt in the 21st Century
 Fatal Imbalance: The Unsuspected Power of the Infinitely Small
 The Great Filter of Evolution: The Key to the Fermi Paradox
 The Last Glacial Shock: The Younger Dryas and Its Impact on Prehistoric Societies
 Why Does the Sunflower Turn Toward the Sun? An Answer Through the Lagrangian
 World Population 2026: Demographic Trends by Continent
 Why Life Emerges from Imbalance and Dies at Thermodynamic Equilibrium
 The Electromagnetic Spectrum and Vision: What Our Eyes Perceive of Our Planet
 Self and Non-Self: A Simplified Physical Reading of Identity
 The Molecular Clock: From Random Mutations to Measuring Time
 The Minimal Cell: The Inevitable Emergence
 White Sands Footprints: America's First Steps
 Hominins: Appearance, Expansion, and Extinctions
 Declining Births: Demographic Catastrophe or Natural Evolution?
 Natural Selection vs. Chance: Why Evolution is Not a Lottery?
 What if Life Originated from Earth? A Revolution in the Theory of Panspermia
 The Great Bifurcation that will Disrupt Our World: Survival or Collapse?
 Primordial Chemistry: Where Do the First Organic Molecules Originate?
 CO and CO₂: Two Gases, Two Risks, Two Biological Mechanisms
 Spontaneous Synchronization: A Universal Phenomenon, from Physics to Life
 Time Challenge: How to Illustrate a Billion Years?
 The Three Essential Components for the Emergence of Life
 Why Did the Genus Homo Nearly Go Extinct 900,000 Years Ago?
 The First Step Towards the Emergence of Life
 The shadow biosphere
 Decline of anthropocentrism: when the cosmos relativizes our importance
 The horseshoe
crab, a living fossil!
 Origin of life
on Earth: Panspermia theory
 Origin of life on Earth: White smoker theory
 Why 37 degrees Celsius?
 Are We Alone in the Cosmos? Between Science and Speculation
 Traces
of Life in the Ice: The Emergence of Prehistoric Mammoths
 The Younger Dryas: The Mini Ice Age That Wiped Out the Megafauna
 The Two Great Ice Ages: Surviving in the Oceans of a Frozen Earth
 Regeneration in Animals Following Amputation: Organic Regrowth
 At the Limits
of Life: Mephisto, Worm of the Infernal Depths
 Discovery
of solid buckyballs in space
 Human Walking:
The Origins of Bipedalism in Hominids
 Karabo: A Window into Human Evolution
 Entropy: What
is Time?
 The
passage between the inert and the living
 The
Great Story of Complexity: From Elementary Particles to the First Organisms
 Megapod uses
volcanic heat
 Ardipithecus:
The 4.4-Million-Year-Old Ethiopian Hominid
 Natural Selection: The Peppered Moth
 The Ordovician:
The Era of Corals, Trilobites, and Graptolites
 Liquid
Water, Much More Than a Solvent: A Catalyst for Chemical Reactions
 Neanderthal:
Humanity's Lost Cousin
 ASIMO: The First
Humanoid
 What conditions allowed the emergence of life?
 Fermi Paradox and Plato's Cave: Are We Alone or Blind?
 Tardigrades:
Indestructible Creatures That Defy the Laws of Biology
 Toumaï: One
of the Oldest Known Hominins
 The
Tree of Life: Billions of Extinct Species and a Single Ancestral Community
 Life
in the Abyss: The Extreme Adaptation of Creatures
 Cyanobacteria
and the Oxygen Crisis: A Primordial Ecological Catastrophe
 From
Matter to Life: The Blurred Frontier of Biological Emergence
 The Smallest Frog in the World: Physiological Secrets of a Microvertebrate
 The explanation of the Little Ice Age
 The Light of Life: A Biosignature Revealed by the Moon
 Living
Light: The Dazzling Secrets of Bioluminescence
 Beyond our senses, the great scientific revolutions
 The
Primordial Soup: Chemical Cradle of Terrestrial Life
 World Population: From One Billion Humans to Demographic Saturation
 Ecology
and Collapse: The Case of Easter Island
 Fractals: Universally Self-Organized
Structures